When the Signal Loses Its Sting: Desensitisation, from Bakery Kitchens to Blue Inhalers
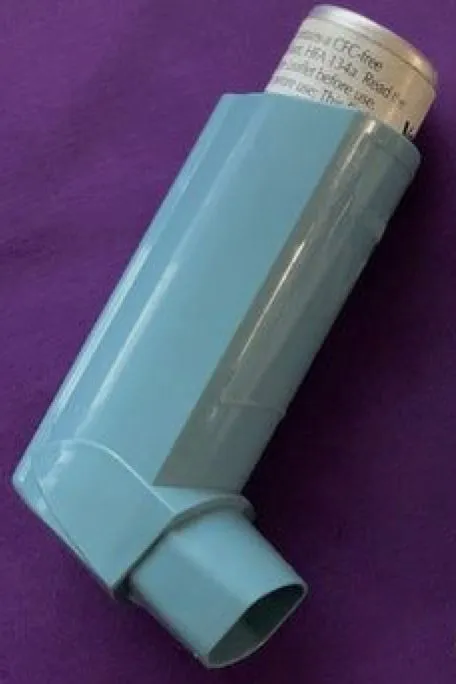
Photo: Fatimah Bello, CC0, via Wikimedia Commons
Walk into any bakery on a Saturday morning and the smell is overwhelming — warm yeast, caramelising sugar, butter in the air. Ten minutes later, you notice nothing. The aroma has not left the room; your nose has simply stopped reporting it. That everyday experience is one of the clearest windows into a process every cell in the body depends upon: desensitisation, the deliberate dampening of a signal that arrives too often or too loudly.
The problem of a message that never stops
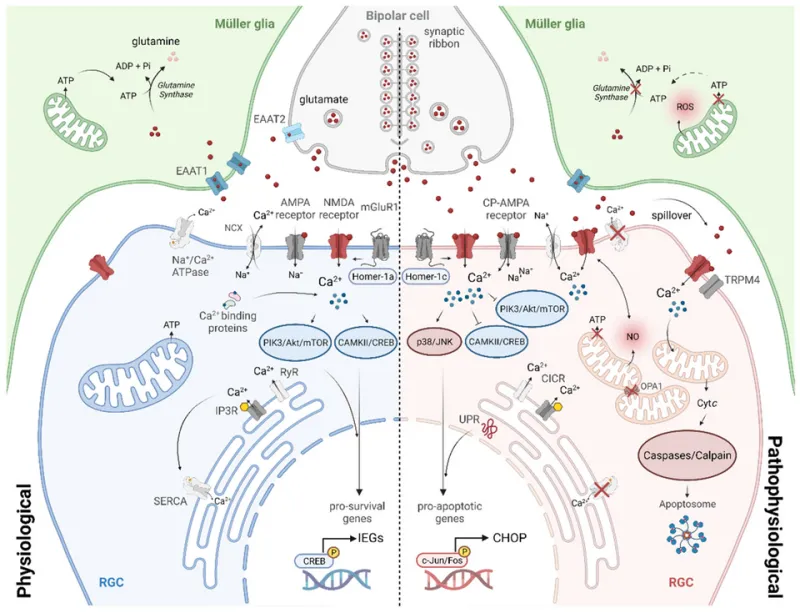
A cell receptor is not a simple switch. When a messenger — adrenaline, an odour molecule, a drug — binds to its receptor, the receptor changes shape and sets off a cascade of events inside the cell. But if the messenger never leaves, the cascade keeps running. Calcium stores drain, energy is consumed, and the cell loses its ability to respond to anything new. Biologically, this would be like a fire alarm that rings at full volume for a week: eventually nobody inside the building can think, and the neighbours stop listening.
Evolution's answer is a suite of mechanisms that collectively turn the volume down without switching the radio off. Neuroscientists call it adaptation; pharmacologists call it desensitisation and, over longer timescales, down-regulation. The distinction matters, and understanding it explains a great deal about how medicines behave in practice.
Phosphorylation: the molecular hand on the fader
The fastest form of desensitisation happens within seconds, and it begins with a phosphate group. Specialised enzymes called G-protein receptor kinases, or GRKs, recognise receptors that have been active for a little too long and attach phosphate groups to them. The phosphorylated receptor is still sitting in the membrane, still exposed to its messenger, but its ability to pass the message onward is sharply reduced.
A second protein family, the arrestins, then physically caps the receptor, blocking its coupling to G-proteins. In many cases, arrestins go further: they act as scaffolds for their own signalling pathways and shepherd the receptor towards the cell's internal disposal routes. What was a blaring loudspeaker a minute ago is now being carried off the stage.
The β₂-adrenergic receptor — the target of salbutamol, the reliever drug dispensed in blue inhalers across Britain — is perhaps the most thoroughly studied example in all of pharmacology. When salbutamol floods the airways during an asthma attack, GRKs and β-arrestin-2 begin their work within minutes. The receptor is phosphorylated, capped, and drawn into the cell inside small membrane pockets called endosomes.
Why the second puff can feel weaker
This molecular choreography has a clinical face. Patients are routinely advised that if their reliever inhaler is needed more and more often, they should seek medical review — and part of the reason is receptor desensitisation. With frequent use, fewer β₂-receptors remain on the airway smooth muscle cell surface available to respond, so each dose of salbutamol has less to grip. The drug has not changed; the receiving apparatus has.
Two processes are at work, and it is worth separating them. Internalisation is rapid and largely reversible: receptors sequestered inside endosomes can be recycled back to the membrane within hours, restoring sensitivity. Down-regulation is slower and more serious: with prolonged exposure, the cell reduces the total number of receptors it makes, degrading existing protein and damping gene transcription. Recovery from down-regulation can take days — which is why long-acting β-agonists are prescribed alongside inhaled corticosteroids, partly to preserve receptor responsiveness over time.
Adaptation in the nose: a quieter kind of forgetting
Olfactory receptors, the ones that tire of the bakery, use a related but distinct strategy. Odorant receptors are also G-protein coupled, and after sustained stimulation, calcium entering through cyclic nucleotide-gated channels activates enzymes that whittle down cyclic AMP — the very second messenger the smell signal relies upon. Calcium also sensitises the machinery that shuts cyclic AMP down. The result is a feedback loop that progressively mutes the nose's output while the odorant is still present.
Crucially, this adaptation is graded and reversible. Step outside for fresh air, and within minutes the same bakery smells overwhelming again. It is a beautifully economical design: the olfactory system keeps its maximum sensitivity for changes in the chemical environment, which are usually the informative part, while ignoring the steady background. The same logic governs how our eyes adapt to a dim pub after a bright high street, and how taste buds stop registering the salt already in our mouths.
Not a flaw — a feature
It is tempting to regard desensitisation as a failure state, a glitch in the machinery. The opposite is true. A cell that could not desensitise would be a cell locked into a single response, deaf to everything else happening around it. Adaptation preserves what engineers would call dynamic range: the capacity to detect and react to new signals of wildly different intensities across time.
For pharmacology, the lesson is profound. A drug is never just a molecule meeting a receptor; it is a molecule entering a system with its own housekeeping, its own faders and off-switches. Prescribing intervals, combination therapies, drug holidays and tolerance warnings all rest, knowingly or not, on the biochemistry of GRKs, arrestins and recycling endosomes.
So the next time the smell of bread fades from the air, or a reliever inhaler seems to offer less than it once did, remember what is happening beneath the surface. The signal has not been ignored. It has been carefully, deliberately, and — in health — reversibly, turned down.